Evolutionary and environmental context of plant energetics
The origins of photosynthetic mechanisms date back over two billion years to ancient cyanobacteria that pioneered oxygenic photosynthesis in primordial aquatic environments. These prokaryotic ancestors fundamentally altered Earth's atmosphere, transforming a reducing environment into an oxygen-rich biosphere that enabled the subsequent evolution of complex multicellular organisms. Today, environmental parameters such as photon flux density, ambient temperature, and atmospheric carbon dioxide concentrations dictate the metabolic efficiency of primary producers across diverse terrestrial and aquatic biomes, shaping global biodiversity patterns and driving vital biogeochemical cycles across the planet.
Geological impact and atmospheric transformation
The proliferation of oxygenic organisms triggered the Great Oxidation Event, precipitating dissolved iron in oceanic ancient waters and steadily building up atmospheric oxygen levels over millions of years. This massive geochemical shift forced anaerobic species into extinction or extreme ecological refugia while paving the way for aerobic respiration and complex animal life.
Climatic adaptations across ecosystems
Different ecological niches and evolutionary pressures have driven the development of specialized metabolic pathways, including C3, C4, and CAM carbon fixation strategies. These physiological adaptations optimize water retention, thermal tolerance, and carbon assimilation under varying moisture regimes, arid environments, and altitudinal gradients.
Mechanisms of Light-Dependent and Light-Independent reactions
The conversion of radiant energy into stable chemical bonds occurs in two primary stages within specialized chloroplast structures: the light-dependent reactions and the Calvin-Benson cycle. Within the thylakoid membrane, pigment complexes absorb photons to excite electrons, driving photophosphorylation and generating adenosine triphosphate (ATP) alongside reduced nicotinamide adenine dinucleotide phosphate (NADPH). These high-energy molecular carriers subsequently fuel enzymatic carbon fixation reactions occurring in the surrounding stroma, ensuring continuous synthesis of organic compounds essential for plant survival and growth.
Photophosphorylation and electron transport chains
Photosystems I and II operate in tandem along the thylakoid membrane, splitting water molecules through photolysis to extract replacement electrons while liberating protons and molecular oxygen gas. The resulting proton motive force across the membrane powers ATP synthase via chemiosmosis, generating chemical energy.
Carbon fixation in the Calvin cycle
Utilizing the ATP and NADPH produced during the light reactions, the critical enzyme ribulose-1,5-bisphosphate carboxylase-oxygenase (RuBisCO) fixes atmospheric carbon dioxide into organic intermediates. This cyclic series of biochemical reactions ultimately yields glyceraldehyde-3-phosphate, which is subsequently converted into glucose and other carbohydrates.
Enzymatic regulation and environmental sensitivity
The operational velocity of the Calvin cycle is tightly regulated by light-induced pH shifts and magnesium ion concentrations in the stroma. This sophisticated regulatory network prevents wasteful nocturnal carbon fixation and synchronizes enzymatic activity with sunlight availability.
Pigment diversity and chloroplast ultrastructure
Specialized internal cellular compartments known as chloroplasts house the intricate biochemical machinery required for efficient photosynthetic transduction. Within these double-membraned organelles, stacked thylakoid disks called grana maximize internal surface area for light capture and electron transport. Chlorophyll a, chlorophyll b, and accessory carotenoid pigments absorb specific narrow wavelengths of the visible light spectrum, ensuring optimal light harvesting across varying canopy conditions, seasonal shifts, and fluctuating light intensities encountered in natural environments by plants.
Thylakoid stacks and grana architecture
The structural organization of grana optimizes spatial arrangement for photon capture, minimizing energy loss through thermal dissipation and maximizing electron transfer efficiency between adjacent photosystems embedded within the membrane matrix.
Accessory pigments and spectral absorption
Carotenoids, xanthophylls, and phycobilins broaden the usable spectrum of electromagnetic radiation by capturing green, yellow, and blue-green wavelengths that primary chlorophyll molecules fail to absorb efficiently, protecting the photosynthetic apparatus from photoinhibition.
How it works
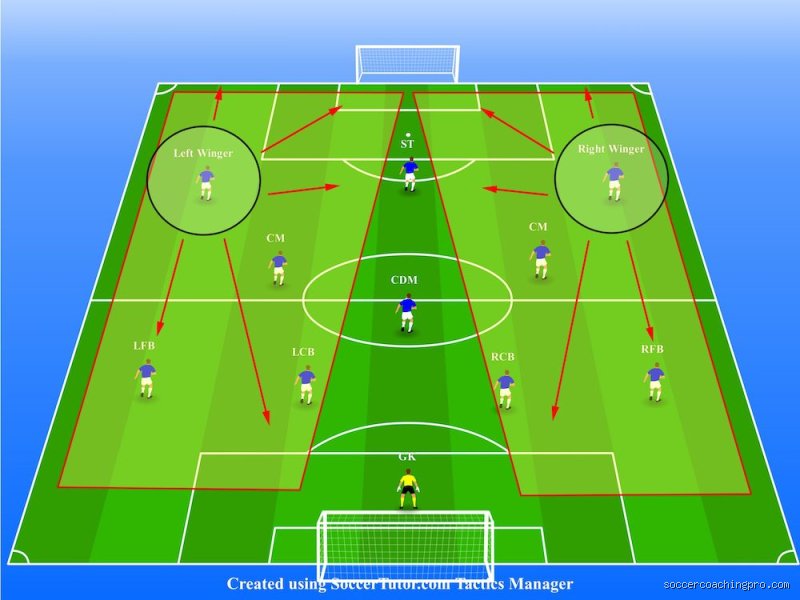
To truly understand whether playing on the flank is advantageous, we must deconstruct the modern tactical demands placed on a wide player. Gone are the days when a wide attacker simply hugged the touchline, waited for a switch of play, and attempted to beat a fullback down the outside before looping a cross into the box. Today's tactical ecosystems—dominated by fluid positional play, half-space exploitation, and gegenpressing—have fundamentally evolved the position.
Modern wide attackers generally fall into two distinct tactical archetypes:
The Inverted Winger: Typically a right-footed player on the left flank or vice versa. Their primary objective is to receive the ball wide, drive diagonally into the central half-spaces, and unleash shots with their dominant foot or combine with central midfielders.
The Traditional Wide Playmaker / Touchline Winger: Players who maintain width, stretch the opponent's defensive block horizontally, and specialize in dynamic 1v1 isolation duels and accurate cutbacks.
Little-Known Aspect
While fans fixate on goals and assists, elite coaching staff value wide players for a hidden metric: press resistance and transitional gravity.
When a team defends deep in a low block, the flank is often the most congested zone because opposing teams shift their defensive structure sideways. A truly elite wide player possesses the unique ability to manipulate this pressure. By receiving passes under intense duress near the sideline and shielding the ball using body geometry, they draw two or three defenders toward them. This gravitational pull completely empties the central corridors of the pitch, creating vast pockets of space for overlapping fullbacks or surging central midfielders to exploit. Understanding this spatial distortion is what separates an average flank runner from a world-class tactical asset.
So, what is the answer?
Weighing the physical demands against the tactical rewards reveals why the position remains one of the most heavily scouted in global football. Playing wide requires an exceptional blend of aerobic endurance, explosive acceleration, and technical composure at high velocities. Unlike central midfielders who operate in 360-degree traffic, wide players often manage restricted angles near the touchline, making decision-making speed paramount.
| Attribute | Traditional Winger | Modern Inverted Winger |
|---|---|---|
| Primary Movement | Vertical (touchline-hugging) | Diagonal (drifting inside) |
| Scoring Profile | Lower volume, assists from crosses | High volume, direct shots |
| Defensive Responsibility | Moderate tracking of fullbacks | High-intensity counter-press |
Final Verdict
So, is playing wide a good position in football? Unquestionably, yes, provided the player matches the mental and physical profile. It offers unmatched opportunities for glory, high individual expression, and tactical influence, as games are frequently won or lost in the wide channels where 1v1 battles decide structural integrity.
Conclusion
Operating on the flank is both a blessing and a rigorous challenge. It demands creativity, unrelenting stamina, and tactical intelligence to adapt to constantly shifting defensive schemes. For players equipped with the right blend of speed, technical skill, and spatial awareness, there is few positions on the pitch more rewarding or influential in shaping the outcome of a match.