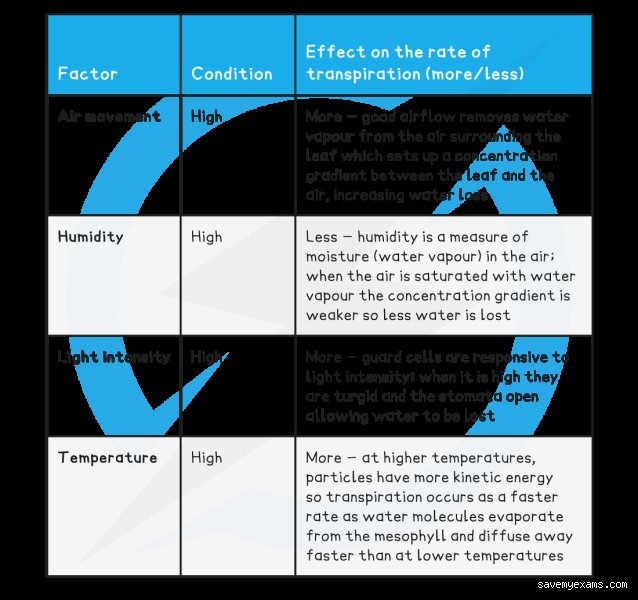
The biophysical mechanics of transpiration
Water movement through a plant operates on a continuous, passive gradient known as the soil-plant-atmosphere continuum. Root systems absorb soil moisture through osmotic gradients, driving water upward through xylem vessels powered predominantly by root pressure and transpirational pull. Transpiration itself relies on evaporation from moist cell walls within the leaf mesophyll into intercellular air spaces, followed by water vapor diffusion down a concentration gradient through microscopic epidermal pores into the surrounding atmosphere.
V
...Building upon the foundational principles of plant water relations and the driving water potential gradients that govern mass flow through the xylem, plants have evolved sophisticated anatomical and biochemical mechanisms to regulate transpirational water loss. While stomatal aperture dynamics provide dynamic, short-term control in response to environmental cues like light intensity and internal CO2 ext{CO}_2CO2 concentration, long-term survival in water-limited environments relies heavily on fixed, intrinsic structural features.
Below is an in-depth exploration of the three primary intrinsic features that fundamentally reduce the rate of transpiration, optimizing water-use efficiency without entirely sacrificing photosynthetic capacity.
1. The development of a thick, impermeable cuticle
The outermost layer of the aerial parts of vascular plants is the epidermis, which is almost universally covered by a protective membrane known as the cuticle. This layer is not cellular; rather, it is an extracellular hydrophobic matrix synthesized by the underlying epidermal cells.
Composition and barrier function
The cuticle is composed primarily of cutin—an insoluble polyester polymer made of hydroxylated and epoxidated fatty acids—impregnated and overlaid with complex mixtures of solvent-soluble lipids known collectively as epicuticular waxes. These long-chain aliphatic hydrocarbons, alcohols, aldehydes, and ketones create a highly hydrophobic surface that acts as the primary barrier against uncontrolled cuticular transpiration.
Resistance to water vapor Diffusion
While stomatal transpiration accounts for the vast majority of water loss when stomata are open, cuticular transpiration occurs continuously across the entire leaf surface, even when stomata are entirely closed. In mesophytic plants living in moist habitats, the cuticle is thin, allowing some residual water loss. However, in xerophytes and species adapted to arid or hyper-saline environments, the intrinsic thickness and crystalline density of the cuticular layer are drastically increased.
By embedding dense, highly ordered layers of epicuticular wax plates or crystalline filaments, the pathway for water vapor diffusion through the epidermis becomes tortuous and chemically hostile to polar water molecules. This structural modification minimizes passive, unregulated water leakage, ensuring that when the plant closes its stomata during severe drought stress, water is effectively locked inside the parenchymatous tissues of the leaf.
2. Stomatal architecture, distribution, and crypts
Stomata are specialized microscopic valves consisting of two guard cells surrounding a central pore (stoma). While essential for gas exchange, allowing CO2 ext{CO}_2CO2 to diffuse into the leaf for photosynthesis and oxygen to escape, they represent the principal site of transpirational water loss, accounting for over 90% of total plant water loss under normal physiological conditions. Plants have therefore evolved profound intrinsic modifications to stomatal architecture and spatial distribution to suppress this loss.
Hypostomatous leaves and stomatal density
A primary architectural adaptation is hypostomatity, where stomata are restricted exclusively to the lower (abaxial) epidermis of the leaf. The upper (adaxial) epidermis, which is directly exposed to intense solar radiation and high ambient temperatures that accelerate evaporation rates, remains entirely non-stomatal and thickly cutinized. Plants under chronic water stress often exhibit significantly lower stomatal densities per unit area, intrinsically limiting the total cross-sectional area available for vapor diffusion.
Sunken stomata and stomatal crypts
In many specialized plants (such as conifers, cycads, and sclerophyllous shrubs), stomata do not lie flush with the leaf surface. Instead, they are recessed into specialized epidermal depressions known as stomatal crypts or chambers.
Micro-climate Boundary Layer: These sunken pits or crypts act as protective micro-pockets. As water vapor diffuses out of the stomatal pore, it becomes trapped within the confined volume of the crypt, creating a localized pocket of high humidity.
Reduced Diffusion Gradient: Because the vapor pressure inside the crypt is significantly higher than the ambient air outside the leaf, the steepness of the concentration gradient (Δc\Delta cΔc) between the sub-stomatal cavity and the external atmosphere is substantially reduced. According to Fick's first law of diffusion, a shallower concentration gradient directly translates to a reduced rate of transpirational water flux.
3. Leaf morphological modifications and surface appendages
Beyond the microscopic properties of the epidermis and stomatal apparatus, the macroscopic and microscopic morphology of the leaf itself plays a critical role in mitigating transpiration. These intrinsic features alter the physical boundary layer resistance and modify the micro-environment immediately surrounding the leaf surface.
Trichomes (Leaf Hairs)
Many drought-adapted species possess dense mats of epidermal outgrowths known as non-glandular trichomes. These microscopic hairs can cover the abaxial or both surfaces of the leaf in a felt-like or woolly layer.
Trichomes function primarily through two mechanisms:
Boundary Layer Enhancement: They trap a stationary layer of humid air immediately adjacent to the epidermal surface. This thick boundary layer increases the diffusion path length for water vapor escaping from the stomata into the rapidly moving turbulent air of the external atmosphere.
Radiation Reflection: Dense white or silvery trichomes reflect a high proportion of incoming shortwave solar radiation. By lowering the net radiation absorbed by the leaf, trichomes reduce leaf temperature, thereby suppressing the vapor pressure deficit (VPD) between the intercellular air spaces and the ambient air, the primary thermodynamic driving force for transpiration.
Reduction of Surface-to-Volume ratio and leaf rolling
Another powerful intrinsic adaptation is the reduction of total transpiring surface area relative to plant volume. Needle-like leaves in conifers, succulent water-storing tissues in cacti, and small, highly coriaceous (leathery) leaves in Mediterranean chaparral species all minimize the absolute area exposed to drying winds and solar heat loads.
In certain grasses (such as Marram grass, Ammophila arenaria), specialized bulliform cells on the upper epidermis lose turgor pressure during periods of severe drought or water deficit. This loss of turgor causes the long, linear leaf blade to roll inward into a tight cylindrical tube. The stomata, which are situated exclusively within the inner grooves of the rolled leaf, are thus sealed inside an insulated, highly humid internal chamber, while the tough, heavily cutinized outer epidermis faces the external environment, effectively shutting down transpirational loss during critical dry spells.
Balancing conservation and carbon assimilation
The evolution of these three intrinsic features, thick cuticles, specialized stomatal architectures like crypts, and protective morphological traits such as trichomes and leaf rolling, highlights the delicate evolutionary balancing act plants must perform.
Every structural modification designed to restrict transpirational water loss simultaneously imposes a degree of resistance to the inward diffusion of carbon dioxide. Consequently