Physiological controls and Environmental constraints: Understanding factors that decrease Transpiration rates in vascular plants
The primary driving force behind transpiration is the water potential gradient along the soil-plant-atmosphere continuum. Water naturally moves from regions of high water potential, such as saturated soil or wet cell walls inside a leaf mesophyll, to regions of low water potential, represented by the dry ambient air. Under conditions where this gradient narrows, equilibrates, or reverses, water loss slows down dramatically. Understanding the specific physical and physiological factors that suppress transpiration allows scientists, agriculturalists, and ecologists to predict plant survival, optimize crop irrigation strategies, and comprehend ecosystem responses to changing environmental parameters.
High relative humidity and atmospheric moisture saturation
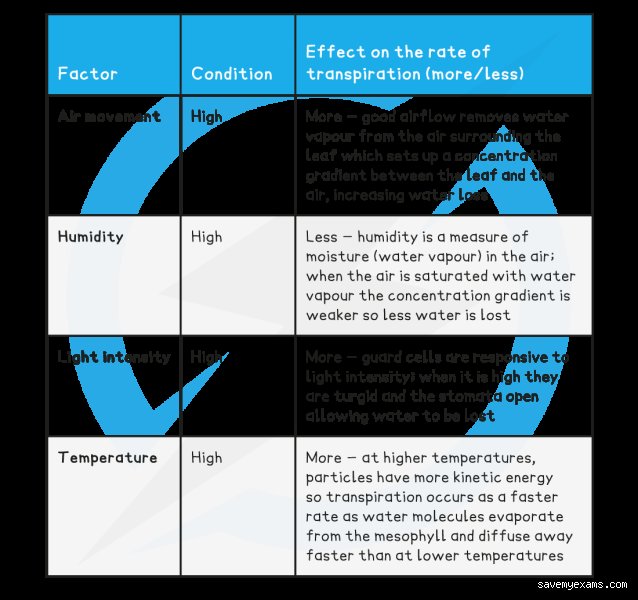
One of the primary environmental determinants governing transpiration is the vapor pressure deficit of the air. Vapor pressure deficit measures the difference between the pressure exerted by water vapor when the air is fully saturated at a specific temperature and the actual vapor pressure of the ambient air. A high vapor pressure deficit indicates dry air with a strong thermodynamic capacity to pull water molecules away from leaf surfaces, accelerating transpiration. Conversely, a low vapor pressure deficit corresponds to high relative humidity, which sharply decreases the rate of transpiration.
When relative humidity approaches one hundred percent, the vapor pressure inside the leaf intercellular air spaces matches the vapor pressure of the external atmosphere. Under these saturated conditions, the driving gradient vanishes entirely. Water molecules cease to diffuse outward through the open stomatal pores at any appreciable rate. In natural settings, this occurs frequently during early morning hours when dew forms, or within dense forest understories and rainforest canopies where air movement is minimal. High atmospheric moisture acts as a direct physical brake on water loss, protecting plants from desiccation during damp weather periods and reducing overall water flux through the xylem network.
Low Temperatures and thermal regulation effects
Temperature exerts a profound influence on transpiration rates through multiple physical pathways, primarily by altering molecular kinetic energy and saturation vapor pressure thresholds. As temperature decreases, the kinetic energy of water molecules inside the leaf mesophyll drops. Lower thermal energy directly reduces the rate of liquid water evaporation from the wet cell walls of the spongy mesophyll into the intercellular air spaces. Consequently, the internal vapor pressure decreases, slowing the overall rate of mass flow out of the leaf structure.
Temperature heavily dictates the saturation point of air. Cold air holds significantly less water vapor than warm air. If ambient temperatures drop rapidly, the relative humidity of the surrounding air increases exponentially unless absolute water content is simultaneously removed. This thermodynamic shift reduces the vapor pressure gradient between the leaf interior and the external environment. In agricultural settings, cooling greenhouses or experiencing sudden cold fronts often suppresses transpiration across numerous crop species, temporarily halting the mass flow of water-borne mineral nutrients from roots to shoots and altering plant metabolic rates.
Stomatal physiology and active closure mechanisms
Beyond passive environmental physics, plants actively regulate transpiration through the precise opening and closing of stomata. Each stoma is flanked by a pair of specialized guard cells that alter their shape based on turgor pressure changes driven by active ion fluxes across cellular membranes. When guard cells accumulate potassium ions and chloride anions from surrounding epidermal cells, water rushes inward osmotically. This influx causes the flexible cell walls to swell and bow outward, opening the pore. Conversely, factors that trigger the loss of these ions cause guard cells to become flaccid, sealing the pore and drastically restricting transpiration.
Several distinct physiological signals induce rapid stomatal closure:
Darkness and Photosynthetic Cessation: In the absence of photosynthetically active radiation, guard cells cease photosynthesis and lose the adenosine triphosphate required to actively pump ions. Consequently, potassium ions exit the cells, water follows via osmosis, and stomata close tightly at night to conserve water when carbon dioxide uptake is unnecessary.
Elevated Intercellular Carbon Dioxide Concentration: When internal leaf concentrations of carbon dioxide rise above optimal cellular thresholds, guard cell membranes hyperpolarize, prompting an immediate efflux of ions and subsequent stomatal closure.
Drought Stress and Phytohormone Signaling: When soil moisture depletes, roots synthesize the phytohormone abscisic acid, which travels via the transpiration stream directly to the leaves. Abscisic acid binds to specific receptors on guard cell membranes, initiating signal transduction cascades that rapidly expel ions, resulting in profound stomatal closure.
Extreme Ambient Temperatures: Excessively high heat can induce severe internal water stress faster than roots can absorb water, prompting plants to close stomata defensively to prevent fatal dehydration, even if soil moisture is initially adequate.
Boundary layer resistance and air movement dynamics
The layer of motionless, humid air surrounding a leaf—known as the boundary layer—plays a critical role in determining transpiration rates. When wind speeds are low or completely absent, transpired water vapor accumulates directly adjacent to the leaf surface, forming a localized microclimate with high humidity. This boundary layer dampens the local vapor pressure deficit, creating physical resistance to further water loss.
To decrease transpiration, a thick boundary layer is exceptionally effective. Leaf morphology often aids this process. Leaves featuring dense trichomes, sunken stomata, or tightly curled structures trap a thick boundary layer of stagnant air, insulating the humid microclimate from external air currents. Without turbulent wind to strip away this humid layer, the local gradient flattens, and transpiration slows down dramatically. Conversely, high wind speeds thin the boundary layer, steepen the gradient, and accelerate transpiration, demonstrating why calm, still air conditions are instrumental in reducing water loss.
Soil water deficit and root Signaling constraints
Although transpiration is primarily governed by atmospheric conditions at the leaf-air interface, soil water availability sets an upper physiological limit on the entire process. When soil water content drops significantly, the soil water potential becomes increasingly negative. This creates a steep resistance gradient that roots must overcome to extract water. As the soil dries, root cells experience mechanical and chemical strain, reducing hydraulic conductivity across root tissues.
Under drought conditions, roots generate hydraulic signals and chemical messengers, including abscisic acid and peptides, that move upward through the transpiration stream before leaves even experience severe dehydration. These root-derived signals induce partial stomatal closure, serving as an early-warning system that dampens transpiration rates long before the plant suffers catastrophic leaf wilting. This proactive down-regulation prevents runaway xylem cavitation, a dangerous phenomenon where water columns break under excessive tension, disrupting the plant's entire vascular transport network.
Physiological mechanisms of stomatal closure under water Stress
When soil water availability drops below a critical threshold, plants activate complex signaling pathways designed to conserve internal moisture. Roots sense the declining water potential and synthesize abscisic acid (ABA), a crucial phytohormone that acts as an early warning messenger. This signaling molecule is transported via the xylem stream directly to the leaves, where it binds to specific receptors located on the plasma membrane of guard cells.
This binding triggers an immediate intracellular cascade, prompting an efflux of potassium ions (K+K^+K+) and anions out of the guard cells. Consequently, water molecules follow the solute gradient and leave the cells through osmosis. As turgor pressure drops rapidly, the guard cells become flaccid, causing the stomatal pore to close tightly. This physiological shutdown drastically curtails water vapor loss, serving as a primary defense mechanism against severe cellular desiccation during dry spells.
The role of Elevated Ambient Carbon Dioxide concentrations
Carbon dioxide (CO2CO_2CO2) concentration in the atmosphere significantly influences stomatal aperture dynamics. Under conditions of elevated atmospheric CO2CO_2CO2, plants often experience partial or complete stomatal closure. Guard cells possess internal biochemical mechanisms that detect intracellular CO2CO_2CO2 levels; an increase signals the plant that sufficient carbon is readily available for the Calvin cycle without requiring wide-open stomata.
Consequently, higher CO2CO_2CO2 levels reduce stomatal conductance across many C3 and C4 plant species. By restricting the size of the opening, the plant limits the outward diffusion of water vapor while maintaining adequate carbon fixation for survival. This interaction highlights how shifting atmospheric chemistry directly alters plant water relations and overall transpiration efficiency.
Boundary layer resistance and air movement dynamics
The boundary layer is a stationary zone of humid air that clings directly to the leaf surface. When the surrounding air is entirely still, water vapor escaping from the stomata accumulates within this micro-environment, reducing the vapor pressure gradient between the internal leaf air spaces and the immediate atmosphere. This reduction in the driving gradient significantly slows down the diffusion rate of water vapor.
While moderate wind can sweep away this humid boundary layer and increase transpiration, extremely calm air or specific structural features that trap the boundary layer, such as dense trichomes or deep leaf grooves, greatly enhance boundary layer resistance. By maintaining a localized pocket of high humidity right outside the stomatal pore, the plant minimizes the driving force required for water loss.
Morphological and anatomical adaptations that restrict Transpiration
Plants inhabiting arid or semi-arid environments have evolved remarkable structural adaptations designed to suppress transpiration permanently or seasonally to survive prolonged droughts.
Thick Cuticles: A waxy, hydrophobic layer covering the epidermal tissue creates a formidable barrier to cuticular transpiration, ensuring that water escapes only through regulated stomatal paths.
Sunken Stomata: Pits or depressions containing stomata create sheltered micro-environments where humidity builds up, effectively decreasing the local vapor pressure deficit.
Reduced Leaf Surface Area: Modifying leaves into spines, needles, or small scales minimizes the total surface area exposed to intense solar radiation and dry air currents.
Trichome Density: Thick mats of specialized epidermal hairs trap a layer of saturated air against the leaf surface, effectively maximizing boundary layer resistance.
Application of antitranspirants in agriculture
In modern agricultural science, managing transpiration is crucial for crop survival during severe drought seasons. Growers frequently utilize chemical compounds known as antitranspirants to artificially decrease water loss without permanently damaging plant health. These substances generally fall into two distinct functional categories:
Film-forming antitranspirants: These chemicals create a physical, semi-permeable polymer barrier over the leaf surface, physically blocking stomatal pores and preventing water vapor escape.
Metabolic antitranspirants: Compounds like abscisic acid analogs or phenylmercuric acetate induce stomatal closure by altering guard cell physiology, achieving water conservation while allowing minimal gas exchange for basic cellular survival.
Summary of factors suppressing Transpiration
To synthesize the intricate network of variables that decrease transpiration, consider the following comparative overview:
| Factor Type | Specific Mechanism | Impact on Transpiration Rate |
|---|---|---|
| Environmental | High relative humidity | Decreases vapor pressure gradient, slowing diffusion |
| Environmental | Elevated atmospheric CO2 | Induces stomatal closure via guard cell signaling |
| Physiological | Abscisic acid (ABA) accumulation | Causes loss of guard cell turgor and stomatal constriction |
| Structural | Thick cuticular wax layers | Blocks passive epidermal water loss |
| Structural | Sunken stomata and trichomes | Enhances boundary layer resistance and traps humidity |
| Agronomic | Application of antitranspirants | Artificially blocks pores or forces physiological closure |
By understanding these multifaceted inhibitory mechanisms, researchers and agriculturalists can better predict plant responses to changing climates and engineer resilient crop varieties capable of thriving under severe water deficits.