To master the culinary arts and optimize kitchen storage, one must look closely at the biochemical ticking clocks embedded inside everyday produce, dairy, and proteins. Some items seem practically immortal on the shelf—dry grains, honey, and salted preserves can outlast civilizations. Conversely, others begin their structural collapse almost the moment they are harvested or separated from their protective husks. This first part of our comprehensive exploration will dissect the fastest-decaying food categories, examining the microscopic catalysts that accelerate decomposition and setting the stage for smarter, science-based preservation strategies.
Why do leafy greens spoil faster than root vegetables?
The speed at which a food item rots is fundamentally tied to its biological origin, surface-area-to-volume ratio, and water activity. Leafy greens such as spinach, arugula, and cilantro represent the absolute vanguard of rapid food spoilage. Unlike dense root vegetables like carrots or beets, which are evolved by nature to store nutrients and moisture safely underground for months, leafy greens are delicate solar collectors designed for rapid transpiration. Once severed from the parent plant, these leaves lose their water supply while continuing to respire actively. Without roots to replenish moisture, the cellular walls begin to collapse, resulting in the dreaded wilted sludge within days of purchase.
Leafy greens possess a massive surface area relative to their weight. This expansive surface invites microbial colonization from airborne mold spores and bacteria like Pseudomonas. Moisture trapped inside plastic grocery bags creates a humid microclimate, accelerating bacterial proliferation and enzymatic browning. Enzymatic activity within the leaf tissue itself breaks down chlorophyll and cell membranes autonomously, even in the cold environment of a refrigerator.
In stark contrast, root vegetables maintain a thick dermal layer—their peel, that acts as a formidable armor against dehydration and microbial invasion. They operate at a much lower metabolic rate in post-harvest storage. While a bunch of spinach might liquefy in five days, a turnip or parsnip can endure for weeks or months under proper conditions. Recognizing this fundamental physiological divide is the first step in rethinking how we shop, store, and consume fresh produce.
The role of ethylene gas in rapid fruit ripening and decay
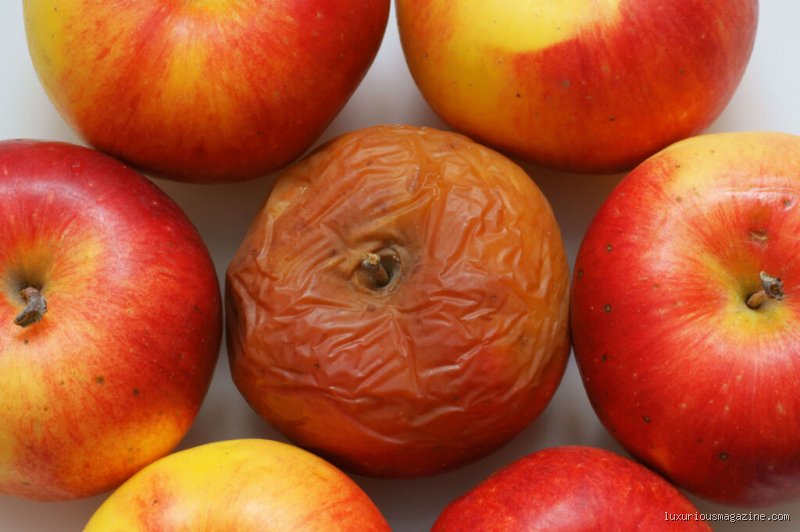
While moisture loss and bacteria doom leafy vegetables, a different invisible enemy orchestrates the rapid decay of many popular fruits: ethylene gas. Ethylene (C2H4C_2H_4C2H4) is a naturally occurring plant hormone emitted as a gas that acts as a chemical messenger, signaling the fruit to initiate ripening, softening, and eventually senescence (aging and rotting). Certain fruits are prolific producers of ethylene, while others are remarkably sensitive to its presence. When high-ethylene producers are housed in close proximity to sensitive items, an accelerated cascade of rot is triggered across the entire fruit bowl.
Consider bananas, avocados, tomatoes, and peaches. These climacteric fruits continue to ripen and produce ethylene after being picked. As ethylene levels spike, starches are rapidly converted into sugars, cell walls are degraded by pectinase enzymes, and the fruit softens into a sweet, highly perishable state. If a bruised apple or an overripe banana is left in a fruit basket alongside sensitive, non-climacteric produce like berries or leafy greens, the ambient ethylene concentration forces those surrounding items into premature decay.
Managing this gaseous catalyst requires deliberate spatial segregation in the kitchen. Storing high-ethylene emitters in breathable containers or utilizing ethylene-absorbing packets can drastically extend shelf life. Ignoring this biochemical interaction, however, guarantees that a single overripe fruit will sacrifice an entire batch of groceries to rapid, mold-driven destruction within 48 to 72 hours.
High-Moisture proteins and dairy: The danger zone of microbial rapid multiplication
Moving beyond the plant kingdom, animal-based proteins and fresh dairy products represent the most aggressive timeline for food rotting, though their decay manifests as bacterial putrefaction rather than fungal mold or enzymatic softening. Foods rich in protein and moisture, such as raw poultry, ground beef, fresh seafood, and unpasteurized soft cheeses, are essentially nutrient-dense culture media for pathogenic and spoilage bacteria alike.
Produce items featuring high water content and delicate cellular structures exhibit rapid decay rates due to several intrinsic biological factors. Berries such as raspberries, blackberries, and strawberries possess minimal protective external barriers. Their skin layers are exceptionally thin and porous, allowing ambient microorganisms direct access to nutrient-rich intracellular fluids. Once harvested, these fruits undergo rapid respiration and moisture loss. Without a robust peel, fungi like Botrytis cinerea easily colonize the surface, initiating gray mold within hours at room temperature.
Leafy greens present an analogous vulnerability. Spinach, arugula, and mixed lettuce varieties have high surface-area-to-volume ratios, maximizing exposure to oxygen and airborne spores. Harvesting severs the root supply, triggering a stress response where the leaves accelerate metabolic processes, consume internal energy reserves, and degrade structural carbohydrates. Pectolytic enzymes break down the middle lamella holding plant cells together, resulting in rapid cellular collapse, wilting, and subsequent sliminess caused by bacterial populations such as Pseudomonas species.
Stone fruits and tropical fruits also deteriorate quickly under specific conditions. Bananas, avocados, and tomatoes produce high volumes of ethylene gas, a natural plant hormone that accelerates ripening and senescence. When stored near ethylene-sensitive items, they induce premature softening and decay across surrounding produce. Tropical fruits lack cold tolerance; refrigeration often triggers chilling injury, disrupting membrane integrity and causing internal browning before standard microbial spoilage can take hold.
Proteins derived from animal sources represent the most hazardous category of rapidly spoiling foods due to their high water activity, neutral pH, and rich nitrogen content. Fresh seafood spoils faster than any other muscle food. Marine microorganisms adapted to cold waters thrive at refrigeration temperatures, continuing metabolic activity even when chilled. Fish flesh contains high levels of trimethylamine oxide, which bacteria rapidly convert into volatile compounds emitting strong off-odors characteristic of spoilage. Nucleotide breakdown also occurs swiftly in fish tissue, reducing freshness indicators within hours of landing.
Ground meats and poultry possess significantly higher surface areas compared to whole muscle cuts. During the grinding process, surface bacteria residing on equipment or outer tissue are distributed throughout the entire product. This aeration and homogenization provide optimal conditions for bacterial strains like Salmonella, Escherichia coli, and Campylobacter to multiply exponentially. Uncooked poultry features a naturally porous skin structure and high moisture content, accelerating both proteolytic bacterial degradation and lipid rancidity.
Cooked starches and prepared meals introduce distinct spoilage dynamics. Cooked rice, pasta, and potatoes left at ambient temperatures enter the temperature danger zone rapidly. Spores of Bacillus cereus, a bacterium commonly found in soil and raw grains, survive standard cooking temperatures. As the food cools, these heat-resistant spores germinate into vegetative cells, producing toxins that cause foodborne illness without necessarily altering the food's appearance or smell.
Dairy items operate on a narrow window between desired fermentation and active spoilage. Raw and unpasteurized milk contains a diverse microflora that rapidly acidifies the liquid by converting lactose into lactic acid. Even pasteurized milk undergoes spoilage driven by psychrotrophic bacteria that survive pasteurization or contaminate the product post-processing. These organisms produce heat-stable lipases and proteases that break down milk fats and proteins, resulting in curdling, bitterness, and putrid aromas.
Soft cheeses such as brie, camembert, and ricotta feature high moisture content and near-neutral pH levels, creating an ideal breeding ground for both beneficial molds and opportunistic pathogens like Listeria monocytogenes. Unlike hard, aged cheeses that lose moisture during prolonged curing, soft cheeses lack the osmotic pressure barrier required to inhibit microbial movement. Consequently, surface spoilage manifests rapidly once cold chain integrity is compromised.
Beyond microbial colonization, chemical reactions dictate how quickly foods rot through intrinsic enzymatic activity and oxidation. Polyphenol oxidase is an enzyme present in many fruits and vegetables, including apples, potatoes, and bananas. When cell walls rupture due to cutting, bruising, or advanced age, this enzyme interacts with phenolic compounds in the presence of oxygen, producing quinones that polymerize into brown pigments. While enzymatic browning does not always indicate immediate microbial rot, it signifies structural degradation and nutrient loss.
Lipid oxidation represents another major pathway of food spoilage, affecting high-fat items such as nuts, seeds, and unrefined oils. Unsaturated fatty acids react with atmospheric oxygen, forming hydroperoxides that subsequently break down into volatile aldehydes and ketones. This chemical process generates rancid odors and acrid flavors, rendering the food unpalatable long before pathogens colonize the matrix. Environmental factors such as light exposure, trace metal presence, and elevated temperatures accelerate this oxidative chain reaction.
Controlling the rate of food rot requires precise management of environmental parameters throughout the supply chain and domestic kitchens. Temperature regulation remains the primary defense mechanism. Lowering storage temperatures reduces microbial respiration rates and enzymatic reaction kinetics according to thermodynamic principles. However, optimal temperature ranges vary significantly; chilling tropical produce causes cellular damage, whereas keeping seafood near the freezing point extends viability.
Atmosphere modification provides another layer of preservation control. Vacuum sealing removes oxygen, suppressing the growth of aerobic bacteria and preventing oxidative rancidity. Modified atmosphere packaging alters the concentrations of oxygen, carbon dioxide, and nitrogen within sealed containers to suppress respiration in fresh produce while inhibiting microbial proliferation. Controlling humidity levels prevents excessive moisture loss in leafy greens while mitigating the condensation buildup that encourages mold growth on delicate berries.
Sanitation protocols at every handling stage minimize initial microbial load. Cross-contamination between raw animal products and ready-to-eat items accelerates spoilage by introducing foreign bacterial strains adapted to rapid reproduction. Utilizing clean cutting surfaces, maintaining strict hand hygiene, and separating ethylene-producing fruits from sensitive vegetables ensure that perishable foods maintain their structural integrity for the maximum duration permitted by their biological properties.